Plant sense
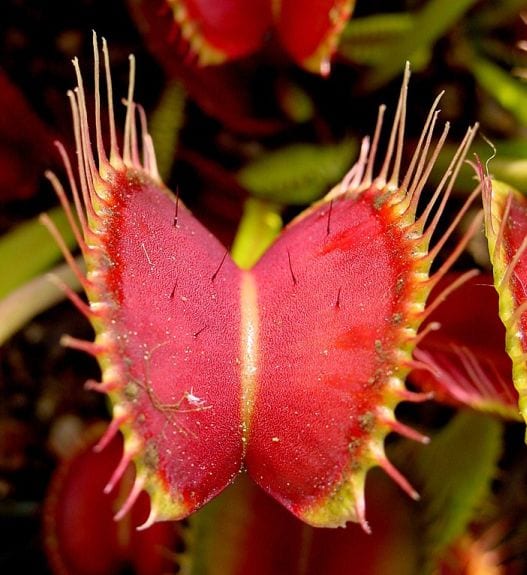
Dionaea muscipula – Venus Flytrap – showing trigger hairs
Plant agency refers to the capacity of plants to regulate behavior through complex systems of communication, coordination, and information processing across multiple scales. Carnivorous plants like the Venus Flytrap captivate us because they make vividly apparent a form of mindless yet goal-directed behavior—an expression of biological agency that distinguishes the living from the non-living. As biological agents, these plants enact the universal and objective imperatives of life—persistence, reproduction, and adaptive transformation (the biological axiom)—through scale-dependent structures, processes, and behaviors shaped by evolutionary history. Their agency does not arise from conscious thought but from a deeply embedded organizational logic that enables context-sensitive responsiveness. From this multiscale, processual form of agency, more elaborate manifestations such as subjective experience and reflective consciousness have emerged in some lineages, including our own.
Several articles explore the idea of biological agency, extending to the realm of plants – first, in a general discussion of plant agency before focusing on plant sensory systems in the article on plant sense while the article plants make sense describes how, as human agency evolved out of biological agency, the evolution of human senses was influenced by plants.
Courtesy Wikimedia Commons
NoahElhardt – Accessed 26 April 2018
Quick Take
From a human perspective, six familiar senses—sight, hearing, touch, smell, taste, balance—are but one evolutionary path. Plants utilize different sensory systems: they detect light, gravity, humidity, chemicals, mechanical disturbance, and electrical signals to regulate growth, adapt physiology, and interact with their surroundings.
Plants possess discernment systems: for example, root systems sense moisture, nutrients, and obstacles; leaves perceive light intensity and quality (e.g. red/far-red detection); tendrils respond to touch. These sensory processes are embedded in distributed chemical, hydraulic, and bioelectrical signaling networks, enabling plants to modulate growth, initiate defense mechanisms, or shift developmental trajectories in context-sensitive ways.
Consider the Venus flytrap: its trigger–hair system and closure mechanism exemplify mindless but goal-directed behavior. When two hairs are stimulated in quick succession, electrical signals trigger the trap’s rapid closure—functioning as a built-in sensory–motor circuit supporting prey capture and nutrient uptake. This illustrates plant sensory capacity without consciousness.
Under the APS model:
Agency underscores that sensing is functional action: plants adjust internal states and external behavior to sustain growth and survival.
Process emphasizes that perception and response are ongoing, self-regulating dynamics, not static or reactive reflexes.
Scale highlights that sensory events operate through nested stages: molecular signal → cellular response → tissue-level behavior → organismal adaptation.
Importantly, APS clarifies that plant sensing is not anthropomorphic analogy. Rather, sensory behavior in plants is functionally equivalent to certain animal perceptual processes, even while depending on distinct material structures. It legitimizes using terms like “perception,” “decision,” and “memory” in non-human contexts—provided they’re grounded in functional similarity, not structural homology.
By revealing how plants interpret environmental information through distributed signaling networks, the article refutes the view of plants as passive or mechanistic. Instead, it portrays them as active agents whose sensory capabilities enable adaptive, context-specific behavior. In effect, plants co-create and respond to their environments in evolutionarily engineered ways.
“Plant Sense” presents a rigorously justified account of plant perception. Using the APS framework, it demonstrates that plants sense, interpret, and act in context-sensitive ways through elaborate multiscale systems—even in the absence of nerves or brains. These sensory behaviors embody the biological imperative and demonstrate functional equivalence with cognitive systems found elsewhere in life.
Introduction
Sensing the World: a broad perspective
When we think about “sensing the world,” we tend to begin with ourselves. Humans commonly recognize six major senses—sight, hearing, touch, taste, smell, and balance—and we use these to interpret and respond to the world beyond our skin. But this familiar list reflects only one particular evolutionary solution. Other forms of life, shaped by radically different bodies and circumstances, have explored a much wider array of ways to access, interpret, and respond to their environments.
How do organisms—especially those without eyes or ears or brains—get their bearings in the world? How do they navigate the challenges of survival, reproduction, and persistence?
Across 3.5 billion years of evolutionary history, life has produced countless solutions to these problems. The organisms that exist today—whether insect, bacterium, or tree—are all heirs to adaptive strategies that worked. Among the most fundamental of these strategies are sensory systems: ways of detecting relevant changes in the external or internal environment and responding appropriately. Though we often associate such systems with animals—particularly motile creatures with nervous systems—this association is misleadingly narrow.
In this article, we explore and compare two divergent evolutionary trajectories: one leading to anatomically modern humans, and the other to flowering plants. These lineages exemplify two distinct but equally successful strategies for engaging the world. Humans, as mobile animals with centralized nervous systems, rely on fast-acting signal transmission, behaviorally coordinated movement, and abstract reflection. Plants, by contrast, are rooted, decentralized, and slow-growing—but they are no less attuned to their surroundings. They sense and respond to gradients of light, moisture, temperature, touch, gravity, and a wide spectrum of chemical signals. Their responses may be enacted through growth, modulation, or internal redistribution of resources—but these are coordinated, adaptive, and often highly specific. In every functional sense, they represent a legitimate, if unfamiliar, form of sensing.
Calling these systems “sensory” is not a metaphor—it is an extension of the biological concept to a wider range of morphologies and strategies. And yet, for much of scientific and popular history, plants have been excluded from discussions of agency, perception, and cognition. This exclusion is not the result of empirical observation, but of linguistic and conceptual bias. We have reserved certain words—communication, memory, intention, learning, value, foresight, self-awareness—for ourselves, or at best for animals that resemble us. These terms have become what might be called difference-talk—a vocabulary that separates rather than connects.
This conceptual boundary has begun to fray. As researchers uncover more about plant behavior, physiology, and responsiveness, it becomes increasingly difficult to deny that plants meet many of the criteria we associate with sentient engagement—even if they do so without brains, neurons, or locomotion. They communicate chemically, modify their behavior based on past experience, and adjust their development in anticipation of future conditions. These are not vague analogies—they are observations grounded in measurable biological function.
Humans are, of course, reflective beings capable of abstraction, symbolic thought, and moral reasoning. As Aristotle remarked over two millennia ago, we are “rational animals.” But we are also biological organisms—evolved, embedded, and continuous with the rest of life. Understanding human sensory experience in this broader evolutionary context does not diminish it. Rather, it allows us to see that the capacity to sense and respond—however differently expressed—is not the exclusive domain of a few privileged lineages. It is a signature of life itself.
This article invites the reader to reconsider what it means to sense the world. By exploring the richly complex sensory lives of plants, we broaden our understanding not only of them—but of ourselves.
1. Introduction: Rethinking Perception in Plants
In the Agency–Process–Scale (APS) framework, perception and cognition are understood as distinct but interrelated functional capacities grounded in biological agency. Perception refers to the ability of an organism to detect and discriminate relevant features of its environment in a context-sensitive manner that contributes to its ongoing organization and survival. Cognition, by contrast, involves the integrated coordination of perception, memory, evaluation, and action over time and across scales, enabling goal-directed and adaptive behavior. Cognition thus includes perception but extends beyond it to encompass more complex functional organization.
The APS framework enables meaningful comparison between human and plant perception through the principle of functional equivalence, which evaluates systems not by structural similarity but by the roles they play in sustaining agency. For example, although plants lack sensory organs or nervous systems, they perceive light, gravity, chemicals, and touch through distributed, highly responsive systems that serve analogous functions to those in animals. By focusing on what a system does—rather than how it does it—functional equivalence supports the claim that plant perception, while structurally distinct, is biologically comparable to that of animals in terms of purpose and effect.
Historical context and conceptual biases
The concept of perception has long been confined within anthropocentric and neurocentric frameworks, shaped by assumptions that locate sensing and awareness exclusively within organisms possessing nervous systems and specialized sense organs. Historically, perception was defined through the lens of human experience, emphasizing consciousness, sensation, and subjective awareness—qualities presumed absent in plants. As a result, the rich sensory capacities of plants have been dismissed or mischaracterized as merely passive or mechanistic reactions.
This bias is rooted in a legacy of dualistic thinking that separates mind from body, and plants from animals, privileging mobility, behavior, and neural complexity as prerequisites for perception. Consequently, plant responses to light, gravity, chemicals, and mechanical stimuli have often been excluded from scientific discussions of perception and cognition, despite their demonstrable adaptiveness and specificity.
To overcome this conceptual limitation, there is a growing need for a biological definition of perception—one that is grounded not in human psychology but in functional and evolutionary terms. Within the Agency–Process–Scale (APS) framework, perception is redefined as the capacity of a living system to detect and respond selectively to environmental information in ways that support its internal coherence and external viability. This shift reframes perception as a processual and agential property of life, distributed across organisms and scales, rather than a mental or neural phenomenon restricted to animals. It allows for a more inclusive and scientifically robust understanding of perception that accommodates the rich sensory worlds of plants and other non-neural organisms.
2. Defining Perception within the APS Framework
In the APS (Agency–Process–Scale) framework, perception is not defined by the presence of a nervous system, specialized organs, or conscious experience. Instead, it is understood as a functional capacity inherent to any agential system—that is, any living system capable of regulating itself in response to internal and external conditions. Perception, in this view, refers to the organism’s ability to detect, discriminate, and integrate environmental cues in a context-sensitive manner that contributes to its adaptive regulation and ongoing viability.
Perception vs. Cognition: A functional distinction
This functional and processual approach distinguishes perception from mere reactivity. Perception involves selective sensitivity: the system must not only receive input but interpret its relevance and act accordingly. For example, plant roots growing toward a moisture gradient are not just passively affected by water; they are actively perceiving and responding in a way that maintains functional integrity. Perception, then, is inseparable from the processes that support the system’s persistence over time.
Cognition, within the APS model, is understood as the extended coordination of perception with memory, evaluation, and action. It encompasses the organism’s ability to integrate information across temporal and spatial scales and to modulate its responses based on prior experience or anticipated conditions. In this sense, cognition subsumes perception but is not synonymous with it.
Crucially, APS treats both perception and cognition as relational and multiscalar: they emerge not from isolated parts but from the integration of processes distributed across the organism. This allows perception to be meaningfully applied to plants, whose sensing is decentralized and embodied through tissues, cells, and chemical networks rather than specialized organs. By focusing on function rather than structure, the APS framework provides a biologically coherent way to understand perception as a basic capacity of life, not a privileged trait of animals.
3. Plant Sensory Modalities
Plants possess a wide range of sensory capacities that enable them to perceive and respond to their environment in precise, coordinated, and functionally meaningful ways. Although lacking eyes, ears, or nerves, plants have evolved highly specialized mechanisms to detect diverse environmental cues—often with a level of sensitivity that rivals or exceeds that of animals.
Light perception in plants is mediated by a suite of photoreceptors (e.g., phytochromes, cryptochromes, phototropins) that detect light intensity, direction, wavelength, and duration. These systems regulate not only photosynthesis but also circadian rhythms, growth orientation (phototropism), flowering time, and shade avoidance, demonstrating finely tuned responses to complex light environments.
Gravitational perception is critical for plant orientation. Specialized cells called statocytes contain dense starch-filled organelles (statoliths) that sediment in response to gravity, enabling roots to grow downward and shoots to grow upward (gravitropism). This directional sensing is dynamically regulated and can adjust to changes in orientation within minutes to hours.
Chemical perception underlies nutrient acquisition, defense, and communication. Plant roots can detect gradients of water, nitrates, phosphates, and other solutes, guiding root architecture toward optimal resource zones. Above ground, plants perceive volatile organic compounds released by neighbors under attack, triggering defensive priming in advance of herbivory. Allelopathic interactions—where plants sense and suppress competitors through chemical signals—further illustrate the discriminating and anticipatory nature of plant chemical sensing.
Mechanical perception allows plants to detect touch, pressure, vibration, and structural load. Tendrils and climbing plants exhibit thigmotropism, coiling in response to physical contact. Plants can distinguish between transient disturbances (like wind) and biologically relevant signals (like an insect landing), responding with different mechanical or chemical defenses.
Temperature and moisture perception are integrated into seed germination, flowering, stomatal regulation, and drought response. Many plants require specific thermal cues to break dormancy, while others regulate water-use efficiency through precise detection of vapor pressure differentials and soil moisture content.
Each of these modalities exemplifies the APS principle that perception is not defined by morphology but by function. The diverse sensing capabilities of plants, distributed across tissues and coordinated over time, demonstrate that perception is a core feature of life—not a privilege of neural animals. These systems enable plants to construct meaningful relationships with their environments, shaping behavior in ways that sustain biological agency.
4. Functional Integration: From Sensation to Action
Perception in plants is not limited to isolated sensory events; it is part of a broader system of functional integration that links environmental input to adaptive response. Within the APS framework, this integration is central to biological agency: to perceive is not merely to register change, but to incorporate it meaningfully into the organism’s self-regulating activity. In plants, this means that sensing is always embedded within coordinated physiological and developmental processes that adjust growth, form, and function to changing internal and external conditions.
For example, root systems exhibit a remarkable ability to sense gradients of water, nutrients, and mechanical barriers. These inputs are processed and translated into differential growth patterns that steer roots toward favorable zones or away from obstacles. The action is not immediate or reactive in a mechanistic sense—it is modulated over time and often involves trade-offs between competing goals (e.g., stability vs. nutrient acquisition), illustrating the evaluative aspect of plant agency.
Above ground, light perception influences not just phototropism but also the timing of flowering, the opening and closing of stomata, and the allocation of energy between growth and reproduction. These responses are mediated by hormone signaling networks—such as auxins, cytokinins, and jasmonates—which function analogously to neural signaling in animals. Although slower and decentralized, these chemical pathways support precise coordination across tissues and scales, integrating perception into systemic responses.
Plants also exhibit forms of memory and priming that further demonstrate functional integration. Prior exposure to drought, herbivory, or temperature extremes can alter future responses, enhancing resilience. These changes are often mediated by epigenetic modifications or alterations in gene expression that persist over time. Such capacity for anticipatory modulation links perception to temporally extended strategies—characteristic of cognitive, rather than purely reflexive, systems.
In APS terms, the integration of sensation and action across spatial and temporal scales is what qualifies perception as agential. It is not the presence of neurons that determines whether perception is meaningful, but whether sensory information is used to coordinate adaptive behavior. Plants, through distributed yet highly organized processes, exemplify this integration. They do not merely react to stimuli—they perceive, evaluate, and act in ways that sustain their organizational coherence and evolutionary success.
5. Functional Equivalence Across Organisms
Comparing plant and animal sensing systems
Functional equivalence’s ability to compare perceptual and cognitive capacities across diverse forms of life. Rather than assessing organisms by structural similarity—such as the presence of a nervous system, brain, or sense organs—functional equivalence evaluates whether different systems perform similar roles in supporting biological agency. If structurally distinct organisms achieve comparable outcomes in sensing, evaluating, and responding to environmental conditions, they can be said to possess functionally equivalent perceptual capacities.
This approach allows meaningful comparisons between human and plant sensing. For instance, both humans and plants perceive light, though through entirely different mechanisms. Humans use retinas and photoreceptive neurons, while plants employ a variety of photoreceptors distributed throughout their tissues. Yet both systems function to guide behavior: in humans, to regulate circadian rhythms and visual navigation; in plants, to direct growth, flowering, and energy use. Despite structural divergence, the functional role—adaptive regulation of activity in response to light—is shared.
The same holds for gravity perception: animals use vestibular systems, while plants use statolith-based sensing in specialized root and shoot cells. In each case, gravitational cues inform directional orientation. Plants and animals also show striking functional analogies in their use of chemical sensing—for foraging, defense, and kin recognition—even though the underlying substrates differ (e.g., neural vs. hormonal pathways).
Importantly, functional equivalence does not imply sameness. It acknowledges differences in structure, speed, and complexity while highlighting the shared organizational purpose of these systems: the regulation of organism–environment relations in ways that support persistence, development, and reproduction. In this view, cognition and perception are not exclusive to animals or tied to consciousness; they are expressions of how living systems maintain coherence over time through selective engagement with their surroundings.
6. Perception Without Neurons: Debunking Myths
A persistent misconception in biology and public discourse is that perception requires a nervous system—and, by extension, that organisms without neurons cannot truly perceive. This view, rooted in anthropocentric and neurocentric assumptions, equates perception with conscious sensory experience and neural processing. However, such a definition excludes vast domains of life, including plants, fungi, and unicellular organisms, all of which demonstrably engage with their environments in structured, purposeful ways.
The APS framework challenges this bias by grounding perception in function rather than form. Perception, in this context, is not about awareness or subjective feeling—it is about the capacity to detect, discriminate, and respond to stimuli in ways that contribute to the regulation of the organism. From this perspective, neurons are one solution among many to the problem of environmental engagement. Plants use chemical, hydraulic, and electrical signaling networks—such as action potentials and calcium waves—to transmit information across tissues and coordinate responses. Though different in speed and structure, these networks fulfill similar roles to neural circuits in animals: integrating sensory input and modulating systemic behavior.
Moreover, the assumption that nervous systems confer superior perception overlooks the profound sensitivity and specificity of plant responses. Plants can detect minute gradients in light, gravity, moisture, chemical signals, and mechanical forces. They respond differentially to touch intensity, distinguish between wavelengths of light, and recognize kin through root-secreted cues. These capabilities are often finely tuned to ecological context, revealing that perceptual sophistication need not depend on rapid locomotion or central processing.
Framing perception as neuron-dependent also obscures its evolutionary origins. Simple sensory–response loops existed long before the emergence of nervous systems. Even bacteria exhibit chemotaxis—moving toward nutrients or away from toxins—based on information processing and feedback regulation. If such capacities are accepted as primitive forms of perception, then plants, with their multicellular coordination and signal integration, clearly possess more complex and functionally rich perceptual systems.
By shedding the myth that perception requires neurons, we open the door to a more inclusive and accurate biology—one that recognizes the distributed, embodied, and evolutionary nature of perception. The APS framework not only supports this reconceptualization but shows that plants, far from being passive or insensate, are dynamic agents actively engaged with their environments through sophisticated, non-neural means.
7. Implications for Cognition and Agency
Recognizing plant perception as a legitimate biological capacity carries significant implications for how we understand cognition and agency across life. In conventional terms, cognition is often equated with mental representation, decision-making, or problem-solving—traits associated with animals, especially those with brains. However, within the APS framework, cognition is defined more fundamentally as the coordinated capacity of a living system to perceive, evaluate, and act adaptively across time and scale. It is not a matter of consciousness but of systemic organization directed toward self-regulation and purposive engagement with the environment.
When perception is acknowledged in plants—not as metaphor but as functionally meaningful—it becomes clear that plants also meet many of the criteria for biological cognition. They discriminate between stimuli, integrate information over time, remember past events, anticipate future conditions, and adjust their behavior accordingly. These capacities emerge not from a central command center, but from a distributed network of signaling systems that modulate plant development, physiology, and behavior in response to internal and external cues.
In APS terms, this distributed organization is itself a form of agential coherence. Cognition, under this view, does not require mental states or symbolic reasoning—it requires the integration of perception, memory, and response in a way that sustains the organism’s viability. Plants exhibit this in myriad ways: from root navigation and canopy competition to stress priming and flowering time regulation. These are not isolated reactions, but context-sensitive, scale-integrated adjustments indicative of agential process.
Importantly, this redefinition of cognition expands our understanding of agency in biology. It challenges the entrenched view that only motile, neuronally endowed organisms are agents, and instead situates agency as a defining feature of life itself—emerging through the capacity to manage complexity, negotiate constraints, and adapt over time. Plants, in this sense, are not passive organisms shaped by their environment; they are active participants in shaping their own developmental trajectories and ecological relationships.
By integrating perception and cognition into a unified processual account of agency, the APS framework offers a biologically grounded alternative to anthropocentric models. It enables a shift from structure-based to function-based thinking, revealing that cognition is not the property of certain kinds of bodies, but a manifestation of how living systems, including plants, enact their ongoing existence.
8. Conclusion: Toward a Unified Biology of Perception
Plant perception, long excluded from mainstream discussions of cognition and sensing, reveals a deeper truth about the nature of life: that the ability to perceive, evaluate, and respond meaningfully to the environment is not a luxury of animals but a requirement of agency. The APS framework reframes perception as a processual, functional capacity—one that is distributed, context-sensitive, and essential to the adaptive regulation of living systems. When freed from anthropocentric and neurocentric constraints, perception can be recognized as a general biological phenomenon, not a privileged faculty of sentient organisms.
Through the lens of functional equivalence, we see that plants, despite their lack of nervous systems, achieve many of the same regulatory outcomes as animals: orienting toward resources, avoiding harm, anticipating environmental changes, and coordinating internal processes to support development and survival. Their perceptual systems—whether responding to light, gravity, touch, chemicals, or temperature—are not primitive substitutes for animal sensing but evolved solutions to the same fundamental problem: how to maintain organizational coherence in a dynamic world.
This recognition challenges the traditional boundaries of cognition and forces a reevaluation of what it means to sense, to know, and to act. Within the APS model, cognition emerges wherever life organizes itself through perception and purposeful responsiveness. Plants, therefore, are not exceptions to cognition—they exemplify it in non-neural, embodied forms that expand our understanding of intelligence in nature.
By adopting a unified biology of perception—one rooted in agency, process, and scale—we move beyond the limiting metaphors of machinery and mind. Instead, we arrive at a more inclusive, evolutionarily grounded perspective in which perception is understood not as a mental attribute, but as a core feature of life itself. Plants, in this framework, are not silent or passive—they are sensing, evaluating, and enacting their worlds. And in doing so, they reveal the richness of a cognitive ecology that transcends the human frame.
Plant Cognition and the APS Framework: A Synthesis
Agency–Process–Scale (APS) offers a unified framework for understanding life as organized through agential, processual, and scale-dependent principles. Plants, as living systems, embody these principles in ways that challenge traditional, animal-centric models of cognition, communication, and behavior. This synthesis integrates key insights from plant science into the APS model.
A – Agency: Plants as Autonomous Biological Agents
- Plants fulfill the biological axiom: the universal, objective, and ultimate disposition to survive, reproduce, and flourish.
- They demonstrate agential autonomy through self-supporting (photosynthesis), self-regulating, self-reproducing, and adaptive behaviors.
- They exhibit goal-directed behavior without the need for consciousness or neural control.
- Plants possess cognitive-like capacities such as sensing, memory, and learning—grounded in evolution, not mental representation.
P – Process: Communication and Integration Without a Brain
- Plant functions are coordinated by distributed signaling processes, not centralized brains.
- Key mechanisms include:
- Hormonal signaling (e.g., auxins, cytokinins) guiding growth and response.
- Electrical impulses transmitted across tissues.
- Chemical signaling using volatile compounds for defense and interaction.
- Mycorrhizal networks enabling interplant communication and cooperation.
- These processes integrate structure, behavior, and internal state toward the plant’s biological goals.
S – Scale: Time, Evolution, and Planetary Influence
- Plants operate across multiple biological scales:
- Short-term: adaptive responses to real-time stimuli.
- Long-term: evolutionary adaptation across generations.
- Global: forming ~99.7% of terrestrial biomass and sustaining all heterotrophic life.
- Their evolutionary longevity and biospheric dominance illustrate planetary-scale agency.
Reframing Cognition and Life
Plant agency demonstrates that intelligence and purposiveness are not exclusive to animals. All living systems capable of coordinated, adaptive, and self-organizing behavior express forms of cognition grounded in the biological axiom.
The APS framework highlights plants not as passive organisms, but as exemplary living systems—models of distributed agency, multiscale coordination, and non-neural intelligence.
On Language and ‘Human-Talk’ in Biology
Describing plant agency often involves terms borrowed from human psychology—such as perception, memory, or anticipation. These terms, sometimes criticized as anthropomorphic, are better understood as instances of ‘human-talk’: the use of human-referent language to capture real, graded similarities between human and non-human organisms. Rather than deny the existence of cognition-like properties in plants, this language reflects the lack of precise alternatives and acknowledges the continuity of function across life forms. When used carefully, human-talk serves not as metaphor but as a kind of verbal homology, signaling shared adaptive functions shaped by evolution. The APS framework supports the responsible use of such language—not to project human traits onto plants, but to recognize that biological agency and cognition are not binary categories. They exist by degree, and understanding them requires terms that reflect this continuum rather than obscure it.
Functional equivalence in plants
Functional Equivalence vs Structural Difference
Although plants and animals differ dramatically in anatomy and behavior, they face many of the same core biological challenges: acquiring energy and resources, responding to environmental changes, avoiding damage, and reproducing successfully. Animals often address these challenges through movement, specialized sense organs, and rapid neural coordination. In contrast, plants rely on their bodies as distributed sensory and response systems—rooted in place yet finely attuned to light, gravity, moisture, touch, chemicals, and even sound.
Rather than centralizing perception in a brain, plants distribute it across tissues and structures that integrate sensing and response at multiple levels of organization. This results in a kind of embodied intelligence: plants grow, reorient, and modulate internal processes to meet environmental demands. These differences in structure do not imply a lack of function. On the contrary, plant responses are often functionally equivalent to animal behavior—achieving similar adaptive outcomes through different means.
This section explores how plants and animals meet shared environmental demands, focusing on functional comparisons that clarify, rather than obscure, their evolutionary distinctiveness.
Consciousness, Sentience, Reality
There seems a vast chasm separating sentient and non-sentient organisms. Human-talk, the mentalistic language we sometimes attribute to plants emphasizes the fact that a plant does not possess a brain or nervous system. Plants are brainless, thoughtless, eyeless, tongueless, noseless, earless, and therefore non-conscious and mindless.
It does not ‘make sense’ to ask ‘What is a plant’s experience of the world like?’ because, without consciousness, there can be no ‘experience’. Plants don’t ‘think’: they also can’t ‘know’, and they don’t ‘feel’. Using this kind of consciousness-talk for plants is metaphorical fantasy at best; just a convenient shorthand way of making scientific investigation more human-like.
And yet, as we shall see, while all of this is true it presents plants to us in an extremely anthropocentric and demeaning way that overestimates the power of conscious deliberation, while at the same time under-rating un-conscious purpose. Remember . . . it was the mindless purposes of un-conscious nature that gave us our bodies and brains in the first place: we humans have not achieved anything remotely so miraculous.
Regarding the biological processes of non-human nature as ‘ignorant’ is just a preliminary error of human judgement. There are many sophisticated structures and processes found in plants that challenge those found in humans because plants, like humans, have successfully adopted their own, albeit very different, strategies (functional adaptations) to survive, reproduce, and flourish under the same broad environmental pressures.
1. Human Perception and Reality
Our understanding of reality is shaped by the sensory and cognitive apparatus unique to our species. What we perceive as “the world” is a human-mediated experience of what is “out there.” This does not mean our view is mistaken or illusory, but it is uniquely human—just one interpretation among many possible experiences of the world.
Despite our remarkable mental capacities, we face cognitive and perceptual limitations. We cannot hear or smell like a dog, see like an eagle, or calculate like a computer. Our reality is different from that of a cow, fish, or plant. While we may excel in abstraction and reason, other organisms outperform us in sensing particular dimensions of the environment. These comparisons highlight that there is no singular reality—only species-specific constructions of the world.
2. Human Consciousness and Its Origins
Human consciousness is extraordinary. Our brains enable hindsight and foresight, complex language, symbolic reasoning, and the construction of vast technologies and societies. These abilities have granted us unprecedented influence over the Earth and other species.
And yet, the brain itself is composed of the same physical matter—“stardust”—as the rest of the universe. What makes it astonishing is its organization: it has become aware of itself. This self-awareness is often admired as the pinnacle of evolution.
But we must not forget that the brain was not designed or built by humans. It is the outcome of mindless evolution—the creative, unreflective power of nature. Nature did not engineer the brain with foresight or purpose. It assembled it from scratch, without consciousness, without planning, and without tools. Compared to this feat, our construction of computers is trivial.
3. Feeling Without a Nervous System?
Plants lack nerves, brains, and the capacity for conscious pain or subjective emotion—but this does not mean they are unfeeling. In animals, feelings arise from sensory signals processed in the brain; in plants, responses to touch, temperature, pressure, and wounding are handled through distributed, non-neural systems. These responses, while not sentient in the animal sense, reflect a kind of non-conscious feeling—the capacity to detect and adaptively respond to physical stimuli.
Examples abound: Venus flytraps use electrical signals to capture prey only after specific contact patterns, while Mimosa pudica folds its leaves in response to touch via ion shifts and water pressure changes. Plants like Arabidopsis alter growth in response to repeated contact (a process known as thigmomorphogenesis), and wounded tomato leaves trigger systemic defense responses using hormonal and electrical signaling.
These behaviors demonstrate that, despite lacking subjective feeling, plants are highly sensitive, physiologically coordinated beings. Their ability to perceive and react is not evidence of sentience or consciousness, but of biologically grounded responsiveness—an essential feature of life’s adaptivity.
4. Consciousness, Sentience, and Plant Agency
To clarify ongoing debates, it is useful to distinguish sentience from consciousness. Sentience refers to the capacity to feel—typically associated with subjective experiences such as pain or pleasure. Consciousness, more broadly, includes awareness of self and surroundings, intentionality, and the ability to integrate information across time and space. Both are normally linked to complex nervous systems and brains.
The idea of plant consciousness fascinates many but remains scientifically unsupported. Some interpretations stretch the meaning of consciousness to include plant responsiveness, memory-like behavior, and communication. But most biologists emphasize that plants lack the neural architectures considered necessary for consciousness or sentience in animals.
What’s often confused in these debates is the distinction between consciousness and agency. Plants are not conscious in the phenomenal or subjective sense, but they are agential: they sense, assess, and act in ways that promote their viability and survival.
The APS (Agency–Process–Scale) framework helps clarify this by shifting the question from metaphysical speculation to functional coherence. Rather than treating consciousness as a binary attribute—something an organism either has or lacks—the APS view treats it as a functional capacity that emerges in some lineages for particular purposes. Plants do not require consciousness to navigate their environments; instead, they employ distributed, non-conscious processes to enact goal-directed, adaptive behavior.
5. Rethinking Anthropocentrism
Language, Metaphor, and Reality
This article examines the ill-defined boundary between conscious and unconscious processes—both in nature and in the language we use to describe it. Our emphasis on uniquely human subjectivity has led us to build linguistic and conceptual barriers between ourselves and other organisms, often coloring scientific assumptions about the nature of reality.
To navigate this terrain, I use scare quotes to signal terms—such as “reason,” “choice,” or “preference”—whose meanings are tightly bound to human consciousness. While such terms may be useful metaphorically, their application to non-human life must be critically assessed.
Ultimately, both humans and plants rely on sensors and feedback systems to interact with their environments. The key difference is that humans interpret this interaction through a lens of self-aware experience, while plants achieve similar functional outcomes through non-conscious, distributed agency. Recognizing this distinction preserves scientific clarity while appreciating the profound diversity of life’s adaptive strategies.
Our brains may admire themselves, but it was evolution—unaware, unguided, and unfeeling—that made them possible. We did not invent consciousness. Nature invented us.
Functional Equivalence and the Senses
Plants and animals face many of the same existential challenges: acquiring resources, avoiding harm, adapting to changing conditions, and ensuring reproductive success. Yet they address these challenges in strikingly different ways. Where animals rely on locomotion, specialized organs, and centralized nervous systems, plants solve similar problems through decentralized, embodied, and temporally extended physiological strategies.
Our tendency to interpret sensory experience through a human lens—what might be called perceptual anthropocentrism—has shaped the way we talk about the senses. This is not necessarily misleading, as long as we remain aware that terms like sight, touch, or hearing are metaphors when applied beyond animals. In what follows, each sense is framed both in its specific human form and in more general biological terms, referring to basic environmental stimuli (such as light, chemicals, or mechanical force) that all organisms must monitor and respond to in order to survive.
From this broader perspective, we see that plants are not passive entities merely adapting to environmental constraints, but active participants in ecological relations—sensing, responding, and transforming their environments. They register gradients of light and gravity, detect mechanical pressure and vibration, respond to airborne and waterborne chemicals, and alter growth patterns accordingly. Though lacking neurons and brains, plants nevertheless translate sensory inputs into coordinated physiological action—regulating development, defence, and reproduction in sophisticated and sometimes surprising ways.
Research in this area remains comparatively underfunded and underexplored—a legacy of long-standing “plant blindness” in both scientific and cultural domains. But this neglect opens up new opportunities. As interest in plant perception grows, young researchers have the chance to make foundational discoveries in a field with deep philosophical implications and wide practical applications—from agriculture and environmental design to robotics and sensory ecology.
1. Plant motility & temporal scale
Motility exposes organisms to diverse environments and plays a central role in how animals interact with the world. In animals, movement depends on locating resources (sensing), transmitting information (nervous system), and coordinating responses (central nervous system). This is often interpreted through an “intentional stance,” where animal behavior appears purposeful.
Plants, in contrast, are generally sessile, but this does not mean they are passive. They respond actively to environmental cues such as light, gravity, touch, moisture, temperature, and chemical gradients. While lacking neurons and muscles, plants exhibit coordinated and adaptive behavior—especially evident through time-lapse imaging, where phototropism, circumnutation, and root navigation suggest purposive responses over longer timescales.
Motility in plants takes other forms: roots grow toward moisture and nutrients; shoots reorient to maximize photosynthesis; flowers track the sun. Some rapid movements (e.g., Venus flytrap closure or Mimosa pudica folding) show plants are capable of swift response mechanisms triggered by mechanical stimulation and bioelectric signals. These are functionally equivalent to sensory-motor coordination, even if structurally different.
Emerging research suggests that plants may also respond to acoustic vibrations. Root growth patterns toward the sound of running water, or pollen release in response to the vibration of bee wings, suggest a capacity for mechanosensory integration that extends beyond classical cues.
Seeing Without Eyes
Sight, or vision, in animals typically refers to the capacity of eyes to detect and focus visible light, generating electrical nerve impulses that the brain processes into mental images—distinguishing shapes, colors, brightness, and motion. Visual perception is more than photoreception; it is the brain’s interpretation of these signals through memory, pattern recognition, and contextual awareness.
Plants, of course, have no eyes and no brains. Yet they are exquisitely sensitive to light. From the standpoint of biological function, seeing can be generalized as the ability to detect and respond to light. In this broader, agential sense, plants can “see”—not subjectively, but functionally.
Light is a fundamental environmental factor, shaping life on Earth in both energetic and informational terms. Our visual systems rely on a narrow band of the electromagnetic spectrum, but humans and other animals also respond to wavelengths outside this range, including infrared and ultraviolet—“invisible light.” Our eyes contain specialized photoreceptors: rods (with rhodopsin) allow for night vision, while cones (with different photopsins) enable color perception in bright light. A fifth receptor, cryptochrome, plays a key role in regulating circadian rhythms.
Plants also possess a diverse array of photoreceptors that allow them to discriminate light intensity, color (wavelength), direction, and duration—critical information for regulating growth, development, and reproduction. In Arabidopsis thaliana, at least 11 distinct photoreceptors are now known to mediate responses such as germination, bending, shade avoidance, photoperiod sensitivity, and more.
One of the earliest scientific insights into plant “vision” came from Charles Darwin’s work with his son Francis in The Power of Movement in Plants (1880). They investigated phototropism—the bending of shoots toward light—and showed that this response is initiated at the tip of the shoot but carried out at a lower region. Subsequent research by Julius von Sachs revealed that blue light triggers this behavior, and we now know that blue-light receptors called phototropins mediate it.
Plants also use light to time life-cycle events. In the early 20th century, researchers found that the duration of light exposure, or more precisely the uninterrupted length of darkness (photoperiod), governs flowering in many species. “Short-day” plants (e.g., soybeans, chrysanthemums) flower as nights lengthen, while “long-day” plants (e.g., barley, irises) require shorter nights. This response is finely tuned: even a brief flash of red light during the dark period can delay flowering, but this effect can be reversed by a pulse of far-red light—mirroring natural twilight conditions.
The molecular key to this red/far-red sensitivity is a single photoreceptor called phytochrome, which exists in two interconvertible forms. Red light activates phytochrome; far-red deactivates it. The location of this sensing is not the shoot tip, but the leaves—demonstrating once again the distributed nature of plant responsiveness.
Other light-sensitive proteins, such as cryptochromes, are shared by both plants and animals. These regulate circadian rhythms and likely originated in early single-celled organisms, helping them anticipate harmful UV radiation. Today, cryptochromes continue to synchronize internal biological clocks across kingdoms of life.
Perhaps the most profound light-related capacity in plants is photosynthesis—the conversion of solar energy into chemical energy. Through photosynthesis, plants not only build and sustain their own structures but support nearly all terrestrial and aquatic life. The energy that powers our own brains and senses ultimately derives from this foundational process.
APS Perspective: Vision as a Distributed Capacity
From the perspective of the Agency–Process–Scale (APS) framework, plant vision exemplifies distributed agency: the ability to perceive and respond to environmental cues without centralized sensory organs. Plants do not have eyes, yet their photoreceptors detect direction, wavelength, and timing of light with astonishing precision. They do not have minds, yet they execute complex decision-making based on this input—whether to grow, bend, flower, or defend.
In this light, seeing is not the exclusive domain of animals with eyes and brains, but a more general biological function: the capacity to extract information from light and act accordingly. By shifting focus from structural similarity to functional equivalence, the APS framework allows us to appreciate plant light-sensing as a form of agential perception—adaptive, coordinated, and evolutionarily significant.
Smelling and Tasting without noses or tongues
Smell, or olfaction, in animals refers to the detection of volatile chemical compounds (odorants) in the air. In humans, the olfactory system begins in the nose, where hundreds of specialized receptors bind to specific molecular features of airborne chemicals. These receptors send electrical signals to the brain, which integrates the information into recognizable perceptions of scent. The result is a complex and often emotionally charged sense, deeply linked to memory and the limbic system. Despite continuing research, the full process by which the brain codes and interprets olfactory information remains only partially understood.
Odors we perceive as singular often consist of many chemicals—for instance, the smell of peppermint contains menthol and over 30 other compounds. Olfactory cues can be conscious (e.g. the recoil from a foul odor) or subconscious, as in the case of pheromones that influence mood, social behavior, and even menstrual synchrony in humans.
By contrast, plants have no nervous system, nose, or brain. But they do detect and respond to airborne chemicals. From a functional perspective, ‘smelling’ is the biological capacity to respond to volatile airborne molecules—a capacity that plants clearly possess, even if the mechanism differs fundamentally from animal olfaction.
One of the most obvious examples of plant use of volatile chemicals is in floral scent. Flowers release perfumes that are attractive or repellent to animal pollinators, depending on ecological context. The sweet smell of jasmine, the putrid odor of the Titan Arum (or “corpse flower”), and the varied scents of fruits and vegetables in a market all reflect this chemically mediated relationship.
The history of plant chemical detection is long. Ancient Egyptians discovered that crushed figs accelerated fruit ripening; the Chinese found that incense smoke had similar effects. In the 1920s, scientists discovered that ethylene, a naturally occurring plant hormone and volatile gas, promotes fruit ripening at extraordinarily low concentrations. By the 1930s, ethylene was recognized as a universal plant signal for ripening and senescence. This not only coordinates fruit ripening within a plant but also acts as a signal to nearby plants and fruit-eating animals.
Ethylene remains the only well-characterized volatile receptor in plants, but other examples suggest additional chemosensory capacities. Parasitic plants such as dodder detect specific volatile compounds from host species (e.g. beta-myrcene from tomato) and grow toward them, while avoiding others (e.g. (Z)-3-Hexenyl acetate from wheat). These responses are highly specific and serve adaptive ecological functions.
Plants can also “warn” each other through airborne chemical signals. Trees attacked by herbivores, for example, release compounds like methyl jasmonate and methyl salicylate. These volatiles are received by neighboring plants, which then pre-emptively activate defense mechanisms. Interestingly, these same compounds are structurally related to plant hormones used in internal immune responses. Methyl salicylate (a volatile) and salicylic acid (a soluble molecule) can be converted back and forth—mirroring the distinction in animals between volatile “smell” molecules and soluble “taste” molecules. In this way, plants “smell” methyl salicylate and “taste” salicylic acid—functionally speaking.
Tasting
Taste, or gustation, is the detection of soluble chemicals. In animals, it is usually associated with the tongue and taste buds. Humans recognize five basic tastes: sweet, salty, sour, bitter, and umami. Taste helps organisms distinguish between nutrients and toxins, guiding feeding behavior and survival. Flavor perception is a multisensory experience, combining taste and smell.
In humans, taste works through molecular binding: specific receptors on taste buds detect chemical compounds in food. For instance, sodium binds to salt receptors, while citric acid triggers sour receptors. This chemical interaction initiates electrical signals that are processed in the gustatory regions of the brain.
In plants, there is no central tasting organ. But functionally, plants also discriminate among soluble chemicals, particularly through their roots. Plants absorb water, mineral nutrients, and chemical messages from soil microbes and neighboring roots. Each plant cell possesses membrane-bound proteins that bind and transport specific ions—calcium, potassium, magnesium, and trace minerals—into the root system. These proteins function as mineral-specific receptors, akin to taste receptors, though they serve both nutritional and signaling roles.
The regulation of this nutrient uptake is complex and tightly coordinated. Water and minerals pass through the root cortex and are selectively admitted into the vascular core by the endodermis, a cellular layer that controls what enters the xylem and phloem—the plant’s internal transport systems. In this sense, plants “taste” nutrients at the surface of the root and again at the gateway to the vascular system, analogous to how human cells maintain mineral balance internally.
Plant ‘taste’ has been central to agriculture. The Green Revolution of the mid-20th century relied on the development of high-yield cultivars responsive to synthetic fertilizers, especially nitrogen, phosphorus, and potassium. These fertilizers worked not by brute force but by engaging the plant’s chemical detection systems—its ability to “taste” and respond to available nutrients. Advances in irrigation, soil chemistry, and genetic engineering continue to depend on our understanding of how plants sense and absorb the resources they need.
Yet as phosphorus and potassium are non-renewable and monocultures threaten resilience, future agriculture must refine—not overpower—plant ‘taste’. Precision nutrient delivery and cultivar optimization will require deeper insight into the sensory capacities of roots, not just the growth responses of shoots.
APS Perspective: Chemosensation Across Kingdoms
Within the Agency–Process–Scale (APS) framework, smell and taste are not fixed by structure (nose, tongue), but defined by function: the ability to detect and respond to environmental chemicals. In this light, both plants and animals engage in chemosensation, though by radically different means.
Plants smell and taste without consciousness or nerves—through distributed, embodied processes that link detection directly to response. Ethylene sensing, volatile-mediated defence signaling, and nutrient-specific uptake are all examples of agential capacities that maintain internal regulation in response to external chemical cues.
APS reframes these sensory capacities not as diminished versions of human abilities, but as evolutionary solutions to similar problems at different scales. Plants do not perceive flavor or odor in the human sense, but they act meaningfully in response to chemical information. Their chemosensation is not representational—it is relational, coordinated, and deeply embedded in their physiology and ecological context.
Hearing without Ears
Sound consists of pressure waves that travel through air, water, or solid matter. Humans hear by detecting these vibrations in the air: the eardrum and hair cells in the inner ear convert changes in air pressure into electrical signals that encode loudness (amplitude) and pitch (frequency), which the brain interprets as sound.
If plants can “see” without eyes, could they also “hear” without ears?
While plants do not have auditory organs, research increasingly shows that they can detect and respond to mechanical vibrations, including some airborne sounds. Studies have demonstrated that certain plants change their growth patterns or defensive chemistry when exposed to specific frequencies. For example, Arabidopsis thaliana has been observed to alter gene expression and release defense chemicals when exposed to the sound of insect chewing, even in the absence of physical contact (Appel & Cocroft, 2014). Similarly, sound frequencies around 200–300 Hz have been shown to enhance germination and growth in some species (Gagliano et al., 2012). These responses suggest that plants possess mechanosensory pathways—using mechanoreceptors or mechanosensitive ion channels—to translate vibrations into biochemical signals, though this is not “hearing” in the animal sense of auditory perception.
Claims that plants enjoy music—whether Mozart or Led Zeppelin—remain anecdotal, with little consistent, reproducible evidence. In many cases, the supposed “preferences” of plants seem to mirror those of the experimenters. What is scientifically supported is that vibrational energy can act as an environmental cue, influencing plant physiology and behavior in specific, testable ways.
In 2000, the genome of Arabidopsis thaliana, a widely studied research plant, was sequenced. The project, involving about 300 researchers and costing roughly $70 million, revealed some 25,000 genes encoded by around 120 million nucleotides. (By comparison, wheat has a similar number of genes but around 16 billion nucleotides; humans have about 22,000 genes in 2.9 billion nucleotides.) Today, entire plant genomes can be sequenced in under a week. Arabidopsis shares many genes with crop plants, making it crucial for agricultural biotechnology. Intriguingly, its genome also contains genes linked to human diseases, just as humans have genes related to plant development—underscoring the evolutionary kinship of life.
Historically, plants may not have evolved specialized auditory organs because, as rooted organisms, they had less need to detect airborne sounds for survival compared to motile animals that rely on hearing for communication, prey detection, or avoiding danger. Nevertheless, vibrations caused by herbivores, wind, or rain could provide cues with real evolutionary value, helping plants anticipate damage, adjust growth, or activate defenses.
A 1973 popular book sensationally claimed plants have emotions, relying on dubious experiments bordering on the occult. While rightly dismissed, it resonated with a human intuition that living nature is purposive, acting as though it has goals or intentions. Today, biological science is more comfortable with teleological language, so long as it is evidence-based. Much of biology involves reverse-engineering—understanding structures and processes in terms of what they are for—without implying conscious thought or human-like feelings.
References
Appel, H. M., & Cocroft, R. B. (2014). Plants respond to leaf vibrations caused by insect herbivore chewing. Oecologia, 175(4), 1257–1266. https://doi.org/10.1007/s00442-014-2995-6
Gagliano, M., Mancuso, S., & Robert, D. (2012). Towards understanding plant bioacoustics. Trends in Plant Science, 17(6), 323–325. https://doi.org/10.1016/j.tplants.2012.03.002
Gagliano, M., Vyazovskiy, V. V., Borbély, A. A., Grimonprez, M., & Depczynski, M. (2017). Learning by association in plants. Scientific Reports, 6, 38427. https://doi.org/10.1038/srep38427
Karban, R. (2015). Plant sensing and communication. University of Chicago Press.
Meyers, J., & Appel, H. M. (2018). Plant responses to mechanical stimuli: Lessons from real and imagined herbivores. Current Opinion in Plant Biology, 44, 14–21. https://doi.org/10.1016/j.pbi.2018.01.004
Volk, T., & Loudon, C. (1985). Plants respond to wind with changes in growth form. Journal of Experimental Botany, 36(6), 744–756. https://doi.org/10.1093/jxb/36.6.744
Drinking
All living organisms need water. Plants use it for photosynthesis, as a medium for chemical transfer, and for maintaining turgour, or rigidity—they wilt when water is scarce. Water also facilitates movement within the plant, transporting nutrients and hormones through the xylem and phloem. On hot days, more water is required because transpiration and evaporation not only sustain metabolism but also have a cooling effect, preventing overheating. The volumes of water involved can be surprisingly large: a single mature oak tree can transpire more than 400 litres of water on a summer day.
Anyone who has cleared drains or seen tree roots lifting paving stones will have noticed how roots sense and grow towards water, a phenomenon known as hydrotropism. Plants achieve this through specialized receptors in root tips that detect differences in water availability in the surrounding soil. These receptors trigger asymmetric growth responses, directing roots toward the wetter side of the gradient (Takahashi et al., 2002). During drought, plants can modify their root architecture, producing deeper and finer roots to explore larger soil volumes, enhancing their chances of accessing scarce water reserves.
Research also reveals that plants communicate water stress belowground. Experiments led by the Novoplansky Research Group at Ben-Gurion University have shown that drought-stressed plants release chemical signals—likely a combination of root exudates and volatile organic compounds in the rhizosphere—that alert neighboring plants to impending water shortages (Novoplansky, 2019). These signals can cause nearby plants to adjust their stomatal opening, growth rate, and even flowering time in preparation for drought, despite not being directly water-stressed themselves. Although the precise chemical messengers remain unidentified, this root-to-root “hydraulic gossip” hints at a sophisticated underground communication network shaping plant communities.
This emerging picture highlights that plants do not passively absorb water. Instead, they actively sense water gradients, regulate their uptake, reconfigure their root systems, and even share drought information with neighbors. Such mechanisms underscore the complex, responsive, and interconnected ways plants manage this vital resource.
References
Novoplansky, A. (2019). Future perception in plants. In: Plant Behaviour and Intelligence (pp. 139–157). Oxford University Press.
Takahashi, N., Yamazaki, Y., Kobayashi, A., Higashitani, A., & Takahashi, H. (2002). Hydrotropism in roots: Sensing of water gradients in the soil and growth response. Plant and Soil, 238(1), 33–39. https://doi.org/10.1023/A:1014267225090
Pierik, R., & Testerink, C. (2014). The art of being flexible: How to escape from shade, salt, and drought. Plant Physiology, 166(1), 5–22. https://doi.org/10.1104/pp.114.239160
Novoplansky, A., Cohen, D., & Sachs, T. (1990). How do plants know when to flower? Plant, Cell & Environment, 13(6), 591–597. https://doi.org/10.1111/j.1365-3040.1990.tb01073.x
Fitzpatrick, C. R., & Schmitt, J. (2019). Environmentally induced plasticity in root architecture enhances drought avoidance in Arabidopsis thaliana. New Phytologist, 224(1), 58–69. https://doi.org/10.1111/nph.15907
1. Human Sensory Orientation and Movement
Touch and the Somatosensory System
Touch is a perception resulting from activation of neural receptors in the skin and hair follicles. These receptors detect variations in pressure (firm, brushing, sustained, etc.). The somatosensory system, distributed throughout the body, processes these stimuli and relays signals to the brain, where they are interpreted as sensations localized to specific body regions.
The Vestibular System: Sensing Gravity and Balance
The vestibular system allows us to perceive our position in relation to gravity and movement. It senses acceleration, body posture, and head orientation using fluid-filled semicircular canals and gravity-sensitive structures called otoliths. These enable us to balance, detect motion (like in an elevator), and differentiate between standing, sitting, or lying down.
Proprioception: Internal Body Awareness
Proprioception is the internal sense of limb position and muscular effort. It allows us to move with coordination—clapping with eyes closed, walking through tight spaces, or adjusting pressure while writing. Proprioceptors located in muscles, tendons, and joints provide this continuous internal feedback.
2. Plant Orientation and Movement
Plant Sensing and Positional Adjustment
Like animals, plants need to orient themselves in space, though they do so without nerves or muscles. They respond to light, gravity, and touch through hormonal and cellular mechanisms. The hormone auxin plays a key role in directional growth. Plants bend toward light (phototropism), send roots downward (geotropism), and may grow around obstacles (thigmotropism).
Statoliths and Gravity Sensing in Plants
Plants use statoliths—starch-filled organelles in root cap or endodermal cells—that settle in response to gravity, much like the otoliths in the human vestibular system. These trigger growth responses that help the plant adjust its orientation. When taken into space, where gravity is absent, plants lose this directional response, underscoring the statoliths’ role.
Historical Experiments: Darwin and Others
From Duhamel’s 1758 observations to Darwin’s seminal The Power of Movement in Plants (1880), scientists have experimentally revealed plant responses to gravity and touch. Darwin showed that the root tip perceives gravity and sends a signal to higher tissues to initiate bending. These insights laid the foundation for understanding plant behavior as responsive and coordinated.
3. Plant Movement Over Time
Circumnutation and Time-Scale Sensitivity
Plants move, but often too slowly for human perception. Darwin documented spiral-like movements called circumnutation, common across plant species. The speed and radius of these movements vary by species and are shaped by genetics and environment. Time-lapse photography reveals these otherwise imperceptible oscillations.
For example, tulip stems circumnutate in 4-hour cycles, wheat in 2. Bean shoots trace a 10 cm spiral; strawberries only a few millimetres. Experiments on the 1983 Columbia space shuttle showed these patterns continue in microgravity, though full expression still depends on gravitational input.
Tropisms and Integrated Positioning
Plants integrate multiple tropic responses—such as phototropism, gravitropism, and thigmotropism—which can counteract or reinforce one another. This coordination enables optimal orientation, much like humans use multiple senses to maintain balance. While we consciously remember our movements, the question arises: can plants remember or store such positional information?
4. Conceptual and Philosophical Reflections
From Sensing to Self-Awareness?
Humans exhibit intention, memory, foresight, purpose, and self-awareness—capacities often associated with consciousness. While plants clearly sense and act, attributing human-like mental states (such as ‘liking’ or ‘preferring’) risks anthropomorphism. Plants do not feel in the human sense, but they do process environmental information and adjust behavior accordingly.
Commentary
Reframing Consciousness: biological purpose to cognitive continuity
The inanimate and animate worlds, the living and the dead, are all made out of the substance of the universe. Living organisms Like us, both plants and animals, are, literally, made out of stardust. But so much depends on the way that this stardust is organized. Organisms are matter that can metabolize, absorbing energy and maintaining a temporary individuality against the forces of inexorable entropy. When continuous replication accompanied by variation occurs in demanding surroundings then those variations that tend to harmonize or ‘fit’ with the environment (functional adaptations) tend to persist. This creates a form of selection but it is not conscious selection, it is natural selection. So far as we can tell this process only happened once so the entire community of life has diverged and radiated from the same biological stock. All organisms are related. Darwin showed that we are not uniquely different and unchanging living beings created separately and placed on earth by God. Instead we are organisms that have arisen out of universal stuff that has acquired the properties of life. And all life, all plants and animals, have evolved by descent from a common ancestor. This means that we humans are not just close relatives of the apes and chimps, we also in a broad biological way, have much in common with plants, as we shall see.
The APS framework situates consciousness not as the origin of agency but as one of its late evolutionary expressions—emerging from deeper biological processes organized around purposive response. This reverses the traditional anthropocentric trajectory that treats meaning and value as the product of human awareness alone. Instead, it supports a graded view of cognition, in which sensing, valuing, and acting evolve through iterative elaborations of functional organization. Plants, on this view, do not need consciousness to be responsive, selective, or goal-directed. By embedding sensory and behavioral capacities within a continuum of natural purposiveness, the APS approach reframes long-standing debates around plant intelligence and consciousness. It allows us to speak meaningfully of plant perception and agency without invoking mental states, recognizing that biological functions carry significance by virtue of their contribution to survival and flourishing. This perspective neither inflates nor dismisses plant capacities but interprets them through a biologically grounded, scale-sensitive account of living systems.
Media Gallery
The development of human consciousness and intellect is usually associated with the evolution of a nervous system and central nervous system that arose in response to the environmental information processing needed when organisms were mobile.
This timelapse video of opening flowers shows that although plants do not change environments, they certainly make the most of their umweldt. We see plants in human animal time – perhaps timelapse allows us to see plants in plant time, including their longer-term purposive mobility.
Key points
short-termism compounds plant blindness by narrowing the narrative of deep time . But plants do behave, they just do it on a different time scale to humans, making it difficult for us to perceive without a great deal of patience.
Agency, Process, Scale (APS)
The Agency–Process–Scale (APS) framework (Spencer, 2025) offers a reimagining of life that places biological agency—the capacity of living systems to regulate, adapt, and pursue functional outcomes—at its center. Rejecting static classifications and anatomical checklists, APS portrays life as a dynamic and multiscale orchestration of purposeful activity, from cells to ecosystems. Where traditional biology leans on mechanistic, bottom-up models and rigid hierarchies, APS emphasizes reciprocal, relational processes that sustain coherence across scales. It seeks not merely to describe what organisms are made of, but to understand what they do to persist and evolve. In contrast to fragmented disciplinary approaches, APS integrates insights from genetics, physiology, ecology, and beyond, uniting them under the functional lens of agency. It reframes cognition, adaptation, and development as expressions of a system’s intrinsic capacity for self-maintenance and evolutionary participation. Rather than reducing biological meaning to molecular mechanisms, APS broadens the scope of inquiry to include plant intelligence, microbial communication, and non-neural cognition—domains often overlooked or marginalized. Ultimately, APS defines life not by structural traits but by its recursive enactment of purposive function across scale, offering a cohesive theory grounded in agential organization and processual integration.
For the APS (loosely):
Agency - the capacity to act
Biological imperative - goal of action
Process - how the goal is pursued
Scale - where/when action occurs
Life, Agency, and the Biological Imperative
What is life? In the Agency–Process–Scale (APS) framework, life is most coherently defined by the biological imperative—the intrinsic tendency of living systems to sustain, adapt, and regenerate their own organized existence across time. This imperative is not a metaphor or heuristic but a scientifically grounded propensity that unifies life’s continuity, coherence, and capacity for evolution.
The biological axiom—that organisms survive, reproduce, adapt, and evolve—describes what life must achieve. The biological imperative explains how: it expresses the internal drive that distinguishes living systems from non-living matter. Unlike any specific structure or trait, the imperative identifies a system-level orientation enacted through sustained, self-organizing activity.
Biological agency is the means by which the biological imperative is realized. Agency is the capacity of a system to coordinate internal processes and environmental interactions in ways that promote its own viability. It is not a fixed trait, but a dynamic, multiscale process—sensitive to context, shaped by evolution, and expressed in behavior. While the imperative defines the condition of being alive, agency defines how that condition is enacted and maintained in practice.
Genes contribute critically by storing and transmitting viable organizational patterns, and natural selection shapes which patterns persist. But neither genes nor selection define life in themselves. The biological imperative precedes them both: life emerges from the capacity to maintain functional coherence in the face of change. Without agency enacting this imperative, there would be no evolutionary process for selection to act upon. In this sense, selection shapes the forms agency takes, but agency underpins the evolutionary process itself.
The most direct manifestation of the biological imperative is behavior—the system-level coordination of perception, regulation, and action aimed at maintaining functional integrity. Such behavior is not confined to movement or sentience, but includes any organized, adaptive response to internal or external change, across all forms of life.
The biological imperative is not an external goal or fixed endpoint, but an emergent, internal orientation: the organized propensity of life to persist, adapt, and regenerate itself. Through this lens, life is defined not by structure or program, but by the agency that enacts this imperative across time. It is this integration of imperative and agency that grounds the APS framework’s naturalized, processual, and scalable theory of life.
Being Mentalistic
The APS framework defines cognition, purpose, and agency as biological capacities—not as mental states or attributes of consciousness. Terms such as memory, decision, or intelligence refer to the functional organization of living systems: their capacity to sense, evaluate, and adaptively regulate internal and external conditions. Similarly, notions like reason and desire are interpreted not as propositional or affective states, but as emergent behavioral patterns grounded in physiological regulation.
APS naturalizes these concepts by interpreting them as evolutionarily grounded, functionally coherent phenomena realized through embodied, goal-directed processes across multiple scales of life. For instance, it is inaccurate to suggest that plants “reason” in a logical or inferential sense. Rather, they display context-sensitive, goal-directed behaviors that are functionally analogous to reasoning, but grounded in their physiological and ecological organization.
Terms like plant neurobiology may emphasize plant signaling processes, but APS cautions against equating these with neural structures or computation. To maintain clarity, the framework prioritizes functional equivalence over structural analogy, underscoring that human mental faculties are elaborations of more basic biological agency—not fundamentally separate. This distinction avoids anthropomorphism while acknowledging cognition as a scalable property of life.
Thus, APS does not deny that plants exhibit intelligent or cognitive-like behavior. Instead, it emphasizes that such capacities—sensing, evaluating, adapting—can be understood as biological functions without invoking mental states or conscious experience. The concern is not whether plants are cognitive, but how cognition is conceptualized and described. Terms like memory or decision are appropriate when used to denote functional and adaptive organization—not introspective thought. In this way, avoiding mentalistic metaphors helps naturalize cognition rather than exclude it.
The broader application of cognitive language to non-human organisms reflects a significant philosophical, semantic, and scientific shift. Philosophically, it challenges human exceptionalism and dualism by framing agency and cognition as embodied, emergent capacities distributed across life. Semantically, metaphors like decision or communication can elucidate biological complexity but require careful use. Scientifically, this shift grounds mentalistic terms in evolutionary and functional processes, revealing how even non-neural organisms engage in regulation, responsiveness, and adaptive behavior. This reconceptualization supports a multiscale, processual view of biology in which cognition is not exclusive to brains but a fundamental aspect of living systems—enabling comparative models while avoiding conflations with consciousness.
Blooming Flower Timelapse
Next Observer – 2019 – 2:40
First published on the internet – 1 March 2019
. . . 3 June 2023 – minor update
. . . 5 August 2023 – Major update in relation to the APS framework
Dionaea muscipula – Venus Flytrap
Showing trigger hairs
Courtesy Wikimedia Commons – NoahElhardt – Accessed 26 April 2018